Plants under salinity stress: a physiological and antioxidant resistance scheme
Shuma Rani Ray ✉
Shuma Rani RayCorresponding author More articles by this author →Aninda Roy
Aninda Roy More articles by this author →
Published
Abstract
Global food output is being negatively impacted by salinity, which is regarded as a major abiotic constraint. Numerous studies have been conducted to identify the methods by which plants tolerate salt stress, and the results have shown some key enzymes and altered biochemical processes that may be responsible for agricultural plants’ resistance. Studies that have been carried out for the last tanners ordinarily have observed the development of salt tolerant cultivars via traditional means, as well as extemporized by modern epoch molecular tools and techniques. Environmental stresses considerably and notably affect the productivity of plants in several ways. Generally, plant growth and development is greatly affected by the process of osmotic stress under soil salinity and Na + and Cl – ions are toxic as well as having injurious effects that results in the imbalance among SO4 2– and Mg 2+ ions as well as significant nutrient elements in plants. As a number of mechanisms reveal the salinity stress response as well as salinity tolerance processes, the effect is called polygenic which includes beneficial compatible solutes or osmolytes, polyamines, reactive oxygen species (ROS) as well as antioxidant defensive processes, transport and compartmentalization of injurious toxic ions. In order to identify the cue factors regarding the particular retaliations or cumulating toxic ions, it is crucial to understand the whole process accountable for growth restriction as well as retarding production of plants with the further span of retaliating the same. The present review will try to summarize the physiological as well as antioxidant defense mechanisms in plants upon salt toxicity. Explaining salinity tolerance as well as its later perspectives and applications in screening for salt tolerance will also be a venture of the present study.
1 Introduction#
In general, the quality and quantity of world agricultural production are greatly diminished by environmental stresses (de Cássia et. al. 2018, Gharsallah et. al. 2016, Foolad 2007, Karan and Subudhi 2012). Besides, 71% crop yield reduction is occurring by abiotic stresses (Ashraf et al., 2010). According to numerous estimation the probable yield reductions are 17% due to drought, 20% due to salinity, 40% due to high temperature, 15% due to low temperature, and 8% due to other factors (, Ashraf & Harris, 2005). Approx. 20 % of irrigated land are affected by the soil salinity which terms as a global complication that both affects and drops crop yields remarkably (Qadir et al., 2014). Most notably, natural salinity and human interferences continuously transforming the arable land is into saline which is anticipated to deluge global effects, that consequence up to 50% land drop within 2050 (Saha et al., 2010; Hasanuzzaman et al., 2013). Salinity stress sometimes called ‘Secrete Murder’ as it destroys plants and other organisms grown on it. ‘White Death’ also used as synonym of it describing white images of lifeless shining lands studded with dead trees. Salinity is one of the most serious problems eradicating global agricultural production (Foolad 2007, Gharsallah al. 2016, Foolad 2007, Karan and Subudhi 2012). It is claimed that, worldwide, 800 million ha of land and 32 million ha of agricultural land are salt-affected (FAO 2015). The closest areas to the seashore are more prone to salinity where salinity reduces agricultural productions to a large scale. Salt problem in agricultural crops, commonly develops in the irrigated areas where salts from the irrigation water build up in the root zone. Irrigated land occupied about 17% of global cultivated land, which merely accords 30% of total crofter production (Hillel, 2000). Crop cultivation under irrigated land is enhancing day by day, which results enhancement of salinity of these lands, creating a major upset for global food reliability. The extremity of Salinity stress inhibits crop production by changing numerous physiological and metabolic activities [Souid et. al. 2018, R. A. James et.al, 2011, A. Rahnama et. al , 2010, Munns, 2005, Rozema et.al, 2008]. Tremendous reduction in Plant growth and yield is caused by several manners under salinity stress.
Sodium Chloride presents as vast percentage in nature playing dominant roles in affecting natural plant production mainly in two consecutive manners: osmotic stress and ionic toxicity. Osmotic pressure occurred more in plant cells compared to surrounding soil solution in absence of salts in soil. On the other hand, osmotic pressure exceeds in soil solution than plant cells under salnity which limits plants ability to absorb water and minerals like K+ and Ca2+ (Glenn, Brown & Khan, 1997; Munns, James & Läuchli, 2006). As Na+ and Cl- has the ability to draw up directly into the cells creating toxic effects on cell membranes, so on the metabolic cytosolic activities (Greenway and Munns, 1980; Hasegawa et al., 2000; Zhu, 2001).
Reduced cell expansion, assimilate production and membrane function, as well as decreased cytosolic metabolism and production of reactive oxygen intermediates (ROSs) are considered as some secondary effects of salinity. Even extremity of salinity can results in plant death. Few plants are able to fight against salinity as well as related stresses by several external and internal mechanisms to evade internal water loss through dehydration and stimulation of sufficient water uptake, amend leaf architecture, amplified extent of assimilates owed to roots, reduced the rate of limb proceeds and developmental rates, dormancy as well as osmotic amendment, etc. (Chaves et al. 2003).
Plants with deep root system, ability to reserve more water-soluble carbohydrates at the base of tiller as well as fast nitrogen uptake, are some superior characters relevant to salt tolerance has been observed in perennial forage grasses in the south of France (Volaire et al. 1998).
Generally, amassing of solutes with low molecular weight as well as inorganic ions are superficial osmotic acclimatizing events to abolish osmotic hazards of the tissue (Gagneul et al. 2007, Ahmad et al., 2010a; Ahmad et al., 2010b; Ashraf & Foolad, 2007; Devi & Prasad, 1998; Foyer et al., 1994). A number of plants in addition to halophytes are able to withstand ion toxicity and sufficient water uptake of even under extremity of salinity (Munns 2002). Osmotic adjustment stabilizes metabolic processes in tissue as well as also enables regrowth upon rewetting (Morgan 1984).
2 Salinity As a Major Curtailment to Plants#
Generally, soil salinity can be occurred and exert its influence on plants in two processes: first present of a high concentration of salts in the soil, that converts it unable for roots to absorb water (osmotic stress), as well as prominence in a high percentage of toxic salts within the plant (ion toxicity). In the outer surface of roots, salts cause reduction of cell growth and metabolism; although, accumulation of toxic salts requires time to exert into plants and after that they become able to affect plant functions (Hasanuzzaman et al., 2013, Munns & Tester, 2008, Gharsallah al. 2016, Foolad 2007, Karan and Subudhi 2012).
The physiological performances of crop plants are considerably as well as adversely affected by salt stress imposition that even turn plant to death as a result of a drastic reduction of growth also due to injury in the metabolic activity(Hasanuzzaman et al., 2013, Gharsallah al. 2016, Foolad 2007, Karan and Subudhi 2012). Usually, the nature of plants, plant species, duration, stage, concentration, as well as mode of salt application to the crops, all are considered as essential factors for estimating the intensity and diminishing effects of salinity to the plants (Dugasa et. al. 2018).
Soil salinity is considered as a serious drastic abiotic stress as it reins majority of crops grown worldwide (Gharsallah al. 2016, Foolad 2007, Karan and Subudhi 2012). Irrigation system and removal of plants from lands may be a reason for it with many other well-known anthropogenic causes (Munns et.al 2008). About 20% of total global cultivable land are now under salinity affected, drastically harassing agricultural production and now it has become a more prominent universal issue (Flowers & Yeo, 1995). Accumulation of dissolved salts within the soil or irrigation water to a harmful concentration causes reduction of plant growth and development referred as salinity stress (Gorham, 1992). Plant growth and developments are largely governed by several physiological processes which are mostly inhibited under salinity needed to be properly scrutinized to understand tolerance mechanisms in plants under salinity (Asgari, 2012). Aggregation of Salts is increased to an extreme level to the plants root zone causing salinity-induced stress (Zhang et al., 2012). For this, reduction in water uptake from soil surface creates water stress, while sufficient water present in the root zone. Water absorption of saline soils requires an extra energy expenditure. Thus, higher salinity will always lead to decreased levels of water as well as inducing analogous stresses like water and osmotic stress (Bauder & Brock, 1992).
High osmotic pressure is created by the high salt concentrations in soil limits water uptake by seeds (Khan & Weber, 2008), responsible for the metabolism of nucleic acid digestion (Gomes-Filho et al., 2008), metabolism of protein changes (Dantas et al., 2007) as well as hormonal offset are aggravated (Khan & Rizvi, 1994), results in the destruction of the ability to utilize seed stores (Othman et al., 2006). There are also varying intramural (plant) and external (natural) processes influencing seed germination under saline conditions incorporating the nature of seed layer, seed torpidity, seedling power, seed polymorphism, seed age, water, gases (Mguis et al., 2013), light and temperature (Wahid et al., 2011). Higher concentrations of the salt results hyper ionic and hyperosmotic stress, even cause’s death of the plant. Membrane layer harm, nutrient unevenness, distorted levels of enzymatic hindrance, developmental regulators and metabolic abnormality, including photosynthesis, which at last prompts plant demise may be occurred from the impact of salinity (Hasanuzzaman et al., 2012; Mahajan & Tuteja, 2005).
Na+ and Cl– ions are the most deleterious for plants under salinity (Tavakkoli et al., 2010). Several complex processes such as photosynthesis is also affected by the biotic as well as abiotic stresses influencing various major components like photosynthetic pigments, photo systems, the electron transport system, CO2 reduction pathways, etc. All kinds of Stresses can affect any of these components, reducing the photosynthetic capacity of plants. Utilization of protein kinases, for example MAPKs and transcription factors are most important to eliminate this harm (Ashraf et al., 2013; Saad et al., 2013; Zhang L et al., 2012).
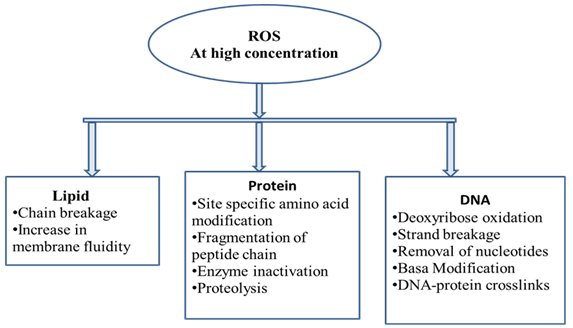
Importance of ion exchange during salinity on the facilitating plant development has observed by Rajendran et al. (2009). They have observed accumulation of hazardous ions after 2–4 weeks of exposure of salt stress. The stress caused by ions (Na+ and/ or Cl– ) overlaps with the osmotic impacts and demonstrates more hereditary variety than osmotic impacts (Dugasa et. al. 2018, Munns et al., 2002).Reactive oxygen species (ROS) induced oxidative spoil to lipids, proteins, in addition to DNA. The cellular hurt takes place in different ways. (Choudhury et. al., 2017, Mursu et al., 2008; Souid et. al. 2018, R. A. James et.al, 2011, A. Rahnama et. al , 2010, Munns, 2005, Rozema et.al, 2008).
3 Plant Species Having Diverse Potentials Under Saline Environment#
Plants are classified as halophytes and glycophytes according to their relevant capacity to sprout under salinity. Halophytes have the intrinsic ability to grow and survive till the entire life cycle under saline environment (around 500 mm NaCl) (Zeng et. al. 2018, Colmer, Flowers & Munns, 2006). On the contrary, Glycophytes are unable to sustain at extreme salt concentration, so also known as non-halophytes. The majority of cultivable crops are glycophytes, but few of them like sugar beet, barley; wheat, etc. has ability to cope with salt to some extent. From another point, halophytes are able to accumulate toxic salts in the leaves in spite of the internal parts to avoid injury as plants are not able to possess a high concentration of salts except slashing (Zeng et. al. 2018, Volkmar et al., 1998). And therefore, these consequences suggest different strategies relating the adaptive mechanisms of halophytes and glycophytes in a distinct manner. Usually halophytes are not able to survive at high level of salinity without balancing the concentrated salt ions as osmoticant materials to some extent. For lack all the above trivial processes, glycophytes are not able to survive in saline conditions whereas halophytes survive. But both the glycophyte and halophyte are equally sensitive to salts if we want to study some sensitive processes like photosynthesis and respiration (Volkmar et al., 1998) under salinity.
4 Retaliations Under Salt Stress (physiological and Oxidative Views)#
Ion homeostasis including compartmentalization, efficient ion transfer and uptake, stimulation of biosynthesis of osmo protectants as well as companionable solutes, inauguration of antioxidant enzyme and synthesis of antioxidant compounds, synthesis of polyamines, production of nitric oxide (NO), and hormone inflection are numerous physiological and biochemical phenomena occurring in plants to withstand extremity of salinity. Several exploration advances elucidating these mechanisms are discussed below.
4.1 Sustaining ionic equanimity#
Some studies reported that adaptive processes of plants under salinity can be elucidated from two points, (1) on the basis of the leaf Na+ concentration and also (2) on the ability of the plant to maintain high cellular Na+ levels (Dugasa et. al. 2018, García-Caparrós et. al. 2018, Shabala and Cuin, 2008). For this, Na/K ratio for both roots and shoots have to be accounted in all cases; although, the ratio is mainly influenced by changing the Na+ concentration, that always posses much greater proportion in comparison to the K+ ion concentration.
The efficiency to uptake crucial ions and their subsequent deliberation, both are fundamental events that require for appropriate growth and development of plants both under normal in addition to salinity (Nikalje et. al., 2018, García-Caparrós et. al. 2018, Niu Xiaomu et. al 1995, Serrano et. al. 1999, Hasegawa, 2013).
The most available form of salt of soil is NaCl, therefore researches needs to be more advanced to comprehend subsequent uptake and convey of Na+ ion within plant body in salinity. The ultimate storage of Na+ ion normally is vacuole where it transported from cytoplasm via Na+/H+ antiporter. Vacuolar type H+-ATPase (V-ATPase) and the vacuolar pyro-phosphatase (V-PPase), are two fundamental forms of H+ pumps of vacuole (Dietz, et.al. 2001, De Lourdes et. al. 2001, and Wang et. al. 2001).
SOS1, SOS2 as well as SOS3 are three crucial proteins in the SOS (Salt Overly Sensitive) signaling pathway also referred as stress signalling pathway in the process of ionic equability and enable plants to survive under salinity.
SOS1 plays an important role in the ion homeostasis through balanced efflux of Na+ ion at cellular level and also in the stimulation of long space convey of Na+ ion from root to shoot. So, higher concentration of this protein stimulate plants tolerance under salinity(Hasegawa et.al. 2000, Sanders et. al. 2000, Shi et. al. 2000, 2002).
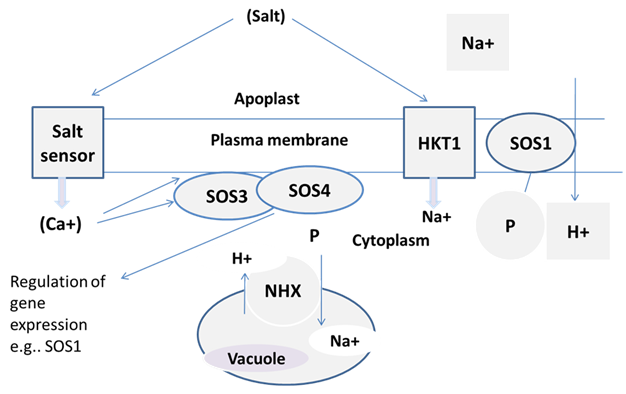
(Source: Nikalje et. al., 2018 , Hasegawa et.al. 2000, Sanders et. al. 2000)
Salt stress-induced Ca 2+ signals are perceived by SOS3 which activates the SOS2 kinase. The SOS3±SOS2 kinase complex regulates cellular Na + levels by stimulating Na + transport out of the cytoplasm (e.g. By increasing the expression and activity of SOS1) and conceivably by restricting Na + entry into the cytosol (e.g. inhibiting HKT1 activity). An additional target of the SOS2 kinase, NHX (vacuolar Na + /H + exchange), also contributes to Na + ion homeostasis by transporting Na + from the cytoplasm into the vacuole.
4.2 High and low-partiality K+ transporters (HKT)#
Several approaches help to keep ionic concentration in a balanced level in the cytoplasm (Ahmad et al., 2010a; Ahmad et al., 2010b; Ashraf & Foolad, 2007; Devi & Prasad, 1998; Foyer et al., 1994). K+ ions play a key regulatory role in promoting Na+ exclusion in plant metabolic process and thus promote the process of osmotic adjustment (Dugasa et. al. 2018, García-Caparrós et. al. 2018, Souid et. al. 2018, Chakraborty et al. 2016). Associated components of membranes usually take part as a crucial role in order to maintain ion concentration in balanced form inside the cytosol under the stress condition for ultimate regulation of ion uptake and transport (Sairam et. al. 2004). The transport phenomenon is carried out by different carrier proteins, channel proteins, antiporters and symporters. Maintaining cellular Na+/K+ homeostasis is pivotal for plant survival in saline environments (R. Munns et. al. 2008, Sairam et. al. 2004, Oh, D.H, et. al. 2010). For appropriate cytoplasmic enzyme activities, it is essential to keep a high concentration of cytosolic K+ which accounts for about 100mM regarded as ideal. The ranges of K+ concentration vary between 10mM and 200mM within the vacuole (R. Munns et. al. 2008, Sairam et. al. 2004, Oh, D.H, et. al. 2010). Vacuole possesse most important and largest plunge of K+ in the plant cell. In order to maintain the turgor within the cell, undoubtedly K+ has a crucial role (R. Munns et. al. 2008, Sairam et. al. 2004, D.-H. Oh, et. al. 2010) that is usually conveyed into the plant cell as opposed to the concentration gradient via K+ transporter and membrane channels. K+ transporters are mediated for K+ uptake mechanisms and possesse relatively high affinity when the concentration of K+ ions are lower outside the cells, on the other hand reverse or low affinity uptake is carried out by K+ channels when the concentration of K+ ions are relatively higher outside the cells,. Availability of K+ ions in the soil can be primarily used to determine the uptake mechanism whereas, very low concentration of Na+ ion (about 1mMor less) usually maintained in the cytosol. As Na+ concentrations are high during salinity stress, it combats with K+ ions during transportation as they are associated with the same transport mechanism and therefore, usually K+ ions decreased (Dugasa et. al. 2018, R. Munns et. al. 2008, Sairam et. al. 2004).
Two classes of HKT family take part either as particular Na+ and K+ co-transporters or Na+ transporters (Hauser & Horie, 2010; Shabala et al., 2010). Improvement of Na+ uptake and higher Na+ levels in xylem sap (salt including conduct) was demonstrated by HKT21 to ameliorate that are analogous with prolonged salt tolerance (Mian et al., 2011a). Na+ avoidance from the shoot is connected with salt tolerance and that genes from the HKT1 subfamily, for example, HKT1;4 and HKT1;5, are included (James et al., 2011; Munns et al., 2012). Shabala et al. (2010) demonstrated that salt exclusion and deliberation both are pivotal for salt tolerance in grain. Actually, grain is an erect demonstration of a harvest which associates halophytic as well as glycophytic belongings, accordingly, both the glycophytic and holophytic components that might be used to adapt to salt stress (Mian et al., 2011b) may be an outstanding model to study.
5 Osmotic Acclimatization#
Several mechanisms assist to fight against disruptive and harmful effects of both primary and secondary stress with the augmentation of osmolytes and antioxidant production (Choudhury et. al., 2017, Ahmad et al., 2010a; Ahmad et al., 2010b; Ashraf & Foolad, 2007; Devi & Prasad, 1998; Foyer et al., 1994; Geebelen et. al., 2002). Compatible solutes such as glycine betaine, proline and poles, etc. which are generally accumulated in the cytoplasm and essential for decreasing water potential occurring in the vacuole and ultimately to make a balance during the ion accumulation in that compartment (García-Caparrós et. al. 2018, Souid et. al. 2018, dos Reis et al., 2012). According to several studies, Salinity stress generally increases compatible organic solutes; however, whether a greater increase in compatible solutes correlates with increased salinity tolerance in plants remains to be shown. For barley, at least, it appears that the more salt-tolerant varieties accumulate less compatible solutes than do the more sensitive varieties (Chen et al., 2007, Mahdavi et. al. 2013).
- Salt ions compartmentalization betwixt the cytoplasm and vacuole provides a strict osmotic gradient across the vacuolar membrane. A Stabilizing process known as osmotic adjustment maintains this flow by an enhancement of the synthesis of chemical and biochemical molecules in the cytoplasm,. As a vital mechanism, Osmotic adjustment is utilized by plants as to fight against salt stress (Pessarakli, 2014, Zhang et al. 2002a). In osmotic adjustment both organic solutes and inorganic ions have a pivotal contribution varying among the captivars, species as well as even among same plant occupying separate positions (Ashraf and Bashir 2003, Ashraf and Foolad 2007). Low molecular weight solutes such as the organic osmolytes traditionally generated in higher plants: sugar and sugar derivatives, such as sucrose, polyols, and heterosides; methylated tertiary N compounds, such as glycine betaine and homarine; amino acids such as proline and glutamate and other low molecular weight metabolites (Jakobsen et al. 2007). Organic osmolytes posses a versatile role in performing osmotic as well as saving sub cellular structure which regards as a central dogma in stress physiology (Hare et al. 1998). Uptake of inorganic ions and osmotic solutes plays as a substitute source compared to the synthesizing organic solutes in plants (Gagneul et al. 2007). Osmotic stress is also experienced in other photosynthetic organisms, considerably in algae mediates similar responses and tolerance mechanisms as higher plants (Chapin 1991). Such as similar compatible solutes (e.g., proline, glycerol, and betaine) are found to be assembled by a unicellular green alga Dunaliella salina (Chlorophyta) and higher plants under salt stressed condition (Zhang et al. 2002b). Proline, glycinebetaine, proline betaine, B-alaninebetaine, D-sorbitol, D-mannitol, sucrose, glucose, fructose, D-pinitol, L-quebrachitol, Myo-inositol, b-dimethylsulphone and propionate are compatible solutes utilized by plants in osmotic adjustment mechanisms (Lauchli & Epstein, 1990).
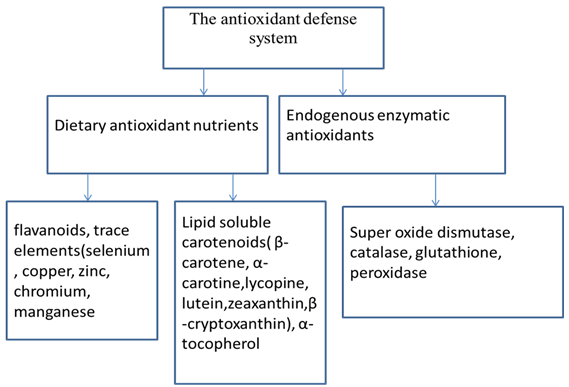
- The antioxidant defense system comprises endogenous enzymatic and exogenous non enzymatic nutrients (Lira et. al. 2018, Choudhury et. al., 2017, Souid et. al. 2018, Zhu et al. 2003). The dietary antioxidant nutrients can either be water soluble or lipid soluble. There are also other dietary constituents that may have either direct antioxidant activity or indirect antioxidant activity such as trace elements that are constituents of antioxidant enzymes (Dugasa et. al. 2018, Alissa et. al. 2012).
Due to expecting compatibility with cytoplasmic entities and processes, normally ‘compatible solutes’ is occasionally used to narrate these organic osmolytes (Munns & Tester, 2008). As an instance, in tobacco proline synthesis plants expand up to 80 times under saline environments.
- Proline is considered as a key amino acid that assists plants to resist osmotic stress (Lira et. al. 2018, Souid et. al. 2018, Rajaravindran et. al. 2012). Generally proline level increases with the consecutive increasing of L-glutamic acid concentration in plants under stresses, hence it is considered as one of the possible precursors for proline biosynthesis(Souid et. al. 2018, Ashraf and Foolad 2007; Kishor et al. 2005, Willekens et al. 1997, Ray et. al., 2016, Rajaravindran et. al. 2012).Various studies reported that the accumulation of proline in a wide variety of species under various kinds of stresses and its possible involvement in adaptive mechanisms (Ray et. al., 2016, Lee et al. 2013, Azad et al. 2012, Marvi et al. 2011, Zhang et al. 2014, da Costa et. al. 2011, Arshi et al. 2012, Turan et al. 2012) . Proline scavenges free radicals to mediate osmotic adjustment as well as stabilizes sub cellular structures (Hare and Cress 1997). For example In durum wheat (Triticum aestivum L.), a positive interaction was observed between proline level and osmotic potential, and thus it was suggested that proline is a crucial metabolite in osmotic adjustment under salinity stress (Poustini et al. 2007). Normally proline accumulates in the cytosol in plants as well as it serves as major factor to the cytoplasmic osmotic adjustment in corresponds to drought or salinity stress (Ashraf and Foolad 2007).
- Glycerol usually emulsed from glucose, serves as principle osmolytes in some plants as well as its rate of synthesis increases upon salinity falls up after which it converts to starch when salinity falls down (Chen and Jiang 2009). However, Glycerol can be an efficient osmolytes under high salinities as it is difficult to match the extreme solubility of glycerol with many other solutes which are compatible and it is chemically inert, so that also non-toxic (Ahmad et. al. 2018). Next, it is an end-product metabolite, and hence its occurrence is unlikely to offset of most of the metabolic processes. Fourth, the energetic cost of glycerol synthesis from glucose is comparatively low and availability of nitrogen doesn’t a matter for it (Chen and Jiang 2009).
- Several sugars such as sucrose, trehalose, glucose and fructose, etc. are the major osmolytes in many plants which are associated with osmotic adjustment. Generally NaCl treatment causes an increase in total sugar content in plant cells, hence the sugar content regarded as a very sentient factor regarding the salt tolerance improvement (Liu and van Staden 2001). Digression of sugars associated with NaCl-tolerance, such as NaCl and Cl– translocation and (or) compartmentalization, solute synthesis for interdependent mechanisms of growth and osmotic adjustment, and protein turn-over Sugars, all play a bit part in the adaptative processes (Liu and van Staden 2001). Sugars are most commonly found to accumulate under osmotic stress in most of the plants. For instance the total soluble sugar level in a salt-tolerant rice variety was more than in the salt-sensitive variety, and thus sugars contribute to the resistance mechanisms to salt-induced osmotic stress in rice plants (Cha-um et al. 2009). Another study revealed that, in root nodules of legumes (Medicago truncatula and Phaseolus vulgaris), the synthesis and accumulation of trehalose was greatly increased as a compatible solute which causes resistancy to salt stress (Lo´pez et al. 2008). Sorbitol is the principle low molecular weight carbohydrate and found to be increased with the extremity of salinity and possesse essential role in the osmotic adjustment as an osmolytes or compatible solute (Eggert et al. 2007a). Another study claimed as mannitol is the main low molecular weight carbohydrate which also observed to be increased upon salinity in red alga Dixoniella grisea (Rhodellophyceae) and claimed to be posses major osmotic functions in the red alga that is unicellular (Eggert et al. 2007b).
- The concatenation of glycine betaine in promoting salinity tolerance has been enumerated in barley and maize (Volkmar et al., 1998) and also verified by several studies from genetic field. Betaines are generally carry a fixed positive charge upon the fully methylated nitrogen atom and are ammonium compounds (Zhang et al. 2002a) which is generally synthesized by many plant families when exposed to saline or drought stress (Munns 2002; Ashraf and Harris 2004; Su et al. 2006). The primary functions of betains is to keep the intracellular and extracellular ions in balanced form through counterbalancing the osmotic potential in order to scale down the toxic effects of salinity as well as also stabilizes the protein structures and play major functions in the protection of the major enzymes, membrane structures, photosynthetic apparatus, cytoplasm, chloroplasts from the toxicity of Na+ and thus regards as a compatible solute also (Raza et al. 2007). Glycine betaine has been also observed in sugar beet (Beta vulgaris L.) to be played a major osmolytic functions (Chołuj et al. 2008) during osmotic stress. Ashraf and Harris (2004) postulated that the most significant determinative of salt tolerance are sustaining as well as accumulating of both K+ and Ca2+, thus K+/Na+ and Ca2+/Na+ ratios can be an efficient and confirmative criteria for selecting salt tolerant crop species (Raza et al. 2007).
- Similarly Mannitol an important osmoprotectant in celery (Tarcynski et al., 1993). Notable extent of carbon is consumed by plants to produce sufficient osmotic substances and this process potentially restricts normal growth and development of the plant (Munns & Tester, 2008). Greater concentrations of inorganic ions also used for osmotic adjustment (Greenway & Munns, 1980).
- Synthesis of organic components in the cell expense more energy than this inorganic approach (Munns & Tester, 2008; Yeo, 1983). Generally, seven moles of ATP are needed in leaf cells, to aggregate one mole of NaCl as an osmoticum,. In contrary, the moles of ATP needed to synthesize one mole of an organic compatible solute are much more. The ATP requirement for the synthesis or accumulation of solutes has been estimated as 3.5 for Na+, 34 for mannitol, 41 for proline, 50 for glycine‐ betaine, and approximately 52 for sucrose (Munns & Tester, 2008). Actually, accumulation of osmoticum, an powerful survival process for plants by adaptation under saline conditions although growth of the plant is greatly affected by it due to ion toxicity and deficiency this mechanism affected (Munns & Tester, 2008; Volkmar et al., 1998).
- Extreme salinity has been observed to stimulate ROS production and accumulation in plant cells (Chawla et al. 2013). Oxidative stress defenses occur through enzymatic antioxidant mechanism including catalase (CAT), superoxide dismutase (SOD), peroxidase (POX) and enzymes of the ascorbate-glutathione cycle as ascorbate peroxydase (APX), monodehydroascorbate dehydrogenase (MDHAR), dehydroascorbate reductase (DHAR) (Dugasa et. al. 2018, Luis et. al. 2018, Foyer and Noctor 2011; Chawla et al. 2013) and non-enzymatic antioxidants as phenolics, flavonoids (Munne´-Bosch 2005; Gupta and Huang 2014; Rakhmankulova et al. 2015; Talbi et al. 2015).
- CAT generally found to be accelerated under salinity stress and associated to the salinity tolerance mechanisms which eliminates toxic levels of H2O2 and renders defense opposed to oxidative stress (Dugasa et. al. 2018, Sudhakar et al. 2001; Bor et al. 2003; Mittova et al. 2003; Mittova et al. 2004; Mittova et al. 2015; Gao et al. 2008 ; Chawla et al. 2013). CAT is involved in scavenging of H2O2 during salt stress and other abiotic stress conditions (Willekens et al. 1997, Ray et. al., 2016, Rajaravindran et. al. 2012, Ediga et. al. 2013, Kong-ngern et al. 2012, Khan et al. 2002, Ahmad et al. 2012, Van Breusegem et al. 2001; Shigeoka et al. 2002, Arshi et al. 2012) and is considered as a major enzyme detoxifying H2O2 in tomato fruits (Murshed et al. 2014).
- Although APX performs the same general function as catalase, it catalyzes the removal of H2O2 by using ascorbate as a reductant (Sudhakar et al. 2001; Bor et al. 2003; Mittova et al. 2003; Mittova et al. 2004; Mittova et al. 2015; Gao et al. 2008 ; Chawla et al. 2013) . APX is a family of isozymes widely involved in regulation of intracellular level of H2O2 in higher plants (Ray et. al., 2016, Rajaravindran et. al. 2012, Ediga et. al.2013, Kong-ngern et al. 2012, Khan et al. 2002, Van Breusegem et al. 2001; Shigeoka et al. 2002, Arshi et al. 2012).
- Several investigations proposed that H2O2 content as well as peroxidase enzymes that generally accumulate in the leaves can be valid criteria to measure the adaptability of crop plants towards salinity stress (Ediga et. al. 2013, Sajjad et. al. 2012, Weisany et al. 2012, Ozdemir et al. 2012, Shaheen et al. 2012).
- GPOX enzymes protect cells against oxidative damage generated by ROS. They catalyze the reduction of H2O2 or organic hydro peroxides to H2O or alcohols. The second category comprises a series of regulatory proteins (transcription factors, protein kinases) involved in the regulation of the signalling cascade that controls the expression of additional genes whose products could belong, in turn, to either of the two groups (García-Caparrós et. al. 2018, Agarwal et al. 2006; Shinozaki and Yamaguchi-Shinozaki 2007)
- Sufficient water uptake requires maintaining an osmotic gradient and thus halophytic plants acquire inorganic ions to a concentration equal to or greater than that of the surrounding solution (Merchant and Adams 2005). In many plants, inorganic ions possess the crucial function in osmotic adjustment than that of compatible solutes and accumulation of organic osmolytes expenses more metabolic energy than sufficient uptake of ions from soil (Patakas et al. 2002).
- Mutant form of rsr1-1 found to be oversensitive to proline in Arabidopsis which can be suppressed by stockpiling of sugar like glucose or sucrose in the medium (Hellmann et al. 2000). So, there may be a straight correlation between proline metabolism as well as sugar-sensing mechanisms. Glycine betaine (5 to 50 mmol/L) found to be an important organic osmolytes to avert proline accumulation in oil seed of rape (Larher et al. 1996). The opposed effect of glycine betaine and the pragmatic consequence relied on glycine betaine uptake and accretion via a feasible osmotic upshot since its endogenous rank was slam to that of proline accumulated in discs incubated in stress media devoid of glycine betaine (Vílchez et. al., 2018). The worth of glycine betaine in reversing the consequence of osmotic distress on the proline reaction has been long-established in leaf discs encumbered with glycine betaine preceding to their incubation in wilting condition. Glycine betaine might have as well amplified the vacuolar assembly in the roots of salt stressed plants for stockpiling additional Na+ in root cells, which was imperative in the uptake of water for plant confrontation to high salt condition ((Vílchez et. al., 2018, Ashraf and Foolad 2007).
Table 1 Most abundant antioxidants that play essential roles in osmotic regulation under salinity stress.
| Antioxidants | Properties | Functions under salinity stress | references |
|---|---|---|---|
| Glutathione (GSH) | Non-enzymatic low molecular weight antioxidant and hydrophilic | Chemically react with free radicals (O2.- , OH.,H2O2 )and scavenges them | Martinez et al. 2018 (Tomato), Hasanuzzaman et al. 2018 (Brassica), Gupta et al. 2018 (highe plants), Broadbent et al. 1995 (Tobacco), Ruiz-Lozano et al. 2018(Rice), Anderson et al. 2004(spurge), Sofo et al. 2015, Nahar et al. 2015 (Mungbean), Das et al. 2014 |
| Ascorbate (AsA) | Non-enzymatic low molecular weight antioxidant and hydrophilic | Chemically react with free radicals (O2.- ,H2O2 )and scavenges them | Golkar et al. 2018 (safflower), Liang et al. 2018 (Kiwifruit), Sofo et al. 2015, Nahar et al. 2015 (Mungbean), Taïbi et al. 2016( Common bean), Jiang et al. 2017(Maize), Alves et al. 2017(Chick pea), Choudhury et al. 2017, Gill et al. 2010, Gupta et al. 2018 (highe plants) |
| Polyphenols | Diverse secondary metabolites and non-enzymatic low molecular weight antioxidant and hydrophilic | Directly scavenge molecular species of active O2 | Golkar et al. 2018 (safflower), Golkar et al. 2018 (safflower), Gul et al. 2018 (Maize), Ashraf et al. 2018 (Maize), Liang et al. 2018 (Kiwifruit), Gupta et al. 2018 (highe plants), Nikalje et al. 2018 (Halophyte), Das et al. 2014 |
| Flavonoids | Non-enzymatic low molecular weight antioxidant and hydrophilic | Scavenger of H2O2 | Ashraf et al. 2018 (Maize), Taïbi et al. 2016( Common bean), Gill et al. 2010, Gul et al. 2018 (Maize), Liang et al. 2018 (Kiwifruit), Gupta et al. Nikalje et al. 2018 (Halophyte)2018 (highe plants), Baskar et al. 2018 (highe plants), Das et al. 2014 |
| Sugar alcohol (eg. Mannitol) | low molecular weight non-enzymatic antioxidant and hydrophilic | Functions as osmoprotectants | Gill et al. 2010, Golkar et al. 2018 (safflower), Gupta et al. 2018 (highe plants), Nikalje et al. 2018 (Halophyte), Das et al. 2014 |
| Tocopherols (vitamin E) | low molecular weight non-enzymatic antioxidant and hydrophobic | Chemically react with free radicals (O2.- , 1O2,OH.,H2O2 )and also scavenges them | Gupta et al. 2018 (highe plants), Kim et al. 2018, Das et al. 2014 |
| Carotenoids | Hydrophobic and non-enzymatic low molecular weight antioxidant | Detoxification of various ROS | Gul et al. 2018 (Maize), Gupta et al. 2018 (highe plants), Nikalje et al. 2018 (Halophyte), Das et al. 2014 |
| Proline | Proline (symbol Pro or P) is a proteinogenic amino acid, organic osmolytes | Acts as an osmoprotectants as able to scavenge ROs | Golkar et al. 2018 (safflower), Vílchez et al. 2018(Pepper), Maghsoudi et al. 2018(Wheat), Gill et al. 2010 ,Hellmann et al. 2000 (Arabidopsis), Wang et al. 2009(alfalfa), Qureshi et al. 2015(Eucalyptus) |
| Glycine betain | Organic osmolytes | Acts as an osmoprotectants | Vílchez et al. 2018(Pepper), Qureshi et al. 2015(Eucalyptus), Joseph et al. 2017, Volkmar et al. 1998 (Barley and Maize), Chołuj et al. 2008 (Sugar beet) |
| Superoxide dismutase (SOD) | Metalloenzyme and low molecular weight antioxidant | Catalyzes the dismutation of O2.- to O2 and H2O2 | Liang et al. 2018 (Kiwifruit), Ashraf et al. 2018 (Maize), Golkar et al. 2018 (safflower), Jiang et al. 2017(Maize), Alves et al. 2017(Chick pea), Choudhury et al. 2017, Gill et al. 2010 |
| Catalase (CAT) | low molecular weight enzymatic antioxidant | Catalyzes the dismutation of two molecules of H2O2 into H2O and O2 | Ashraf et al. 2018 (Maize), Liang et al. 2018 (Kiwifruit), Golkar et al. 2018 (safflower), Sofo et al. 2015, Nahar et al. 2015(Mungbean), Taïbi et al. 2016( Common bean), Zhao et al. 2017(Arabidopsis), Jiang et al. 2017(Maize), Alves et al. 2017(Chick pea), Choudhury et al. 2017, Wang et al. 2009(alfalfa), Gill et al. 2010, |
| Peroxidasa (POD) | Heme containing protein and enzymatic antioxidant | Oxidizes aromatic electron donor such as guaicol and pyragallol at the expense of H2O2 | Sofo et al. 2015, Liang et al. 2018 (Kiwifruit), Nahar et al. 2015 (Mungbean), Taïbi et al. 2016( Common bean), Jiang et al. Golkar et al. 2018 (safflower), 2017(Maize), Alves et al. 2017(Chick pea), Ashraf et. al. 2018 (Maize), Choudhury et al. 2017, Wang et al. 2009(alfalfa), Gill et al. 2010, Gul et al. 2018 (Maize) |
| Ascorbate peroxidase (APX) | low molecular weight enzymatic antioxidant | Reduces H2O2 to H2O by using two molecules of AsA and generates monodehydroascorbate (MDHA) | Liang et al. 2018 (Kiwifruit), Ashraf et al. 2018 (Maize), Sofo et al. 2015, Nahar et al. 2015(Mungbean), Taïbi et al. 2016( Common bean), Jiang et al. and Golkar et al. 2018 (safflower), 2017(Maize), Alves et al. 2017(Chick pea), Choudhury et al. 2017, Wang et al. 2009(alfalfa), Gill et al. 2010 |
| Glutathione peroxidase (GPX) | enzymatic antioxidant | Reduces H2O2 to H2O and also organic peroxides | Anderson et al. 2004(spurge), Bela et al. 2015(Arabidopsis), Diao et al. 2014(Rice), Gao et al. 2014(Arabidopsis), Sofo et al. 2015, Nahar et al. 2015(Mungbean), Taïbi et al. 2016( Common bean), Wang et al. 2009(alfalfa), Gill et al. 2010 |
| Glutathione reductase (GR) | NADP(H) dependent enzymatic antioxidant | Reduces GSSG to GSH | Anderson et al. 2004(spurge), Sofo et al. 2015, Nahar et al. 2015(Mungbean), Taïbi et al. 2016( Common bean), |
6 Conclusion#
Environmental stresses menace plant development, growth also yield and these intimidations are key apprehensions of the human internationally. By means of expansion in population, additional food production is obligatory to congregate global supplies excluding abiotic and biotic stresses lock up its yield. But, amongst all stresses, salinity is the chief distressing since it is prevalent in both arable as well as non-arable lands. The consequences of extreme salts have been pragmatic to have a catastrophic consequence ahead approximately all plants. Therefore, it is decisive to comprehend the cellular mechanisms that take place in plants in saline environment in the trust of ruling an integrated explanation to contest such tribulations. Biotechnology holds pledge for both aspects:
(1) through the most recent tools and techniques, comprehensive studies can be approved away to comprehend the processes inside the cell in different circumstances; in addition to (2) the included prospective of biotechnology can be engaged to contest such harms through changing the hereditary stuffing or by appearance patterns or by optimizing the biochemical with molecular pathways in lots of ways.
Declarations
♥Acknowledgements
Article information
- Published
Copyright © 2025 Shuma Rani Ray. This is an open access article distributed under the Creative Commons Attribution License, which permits unrestricted use, distribution, and reproduction in any medium, provided the original work is properly cited. CC BY 4.0 · Corrections policy
References 163#
- 1
Alscher, R.G., Erturk, N. and Heath, L.S., 2002. Role of superoxide dismutases (SODs) in controlling oxidative stress in plants. Journal of experimental botany, 53(372), pp.1331-1341.
- 2
Arbona, V., Hossain, Z., López-Climent, M.F., Pérez-Clemente, R.M. and Gómez-Cadenas, A., 2008. Antioxidant enzymatic activity is linked to waterlogging stress tolerance in citrus. Physiologia Plantarum, 132(4), pp.452-466.
- 3
Arshi, A., Ahmad, A., Aref, I.M. and Iqbal, M., 2012. Comparative studies on antioxidant enzyme action and ion accumulation in soybean cultivars under salinity stress. Journal of environmental biology, 33(1), p.9.
- 4
Alves Lara Silva Rezende, R., Rodrigues Soares, J.D., dos Santos, H.O., Pasqual, M., Braga, R.A., Reis, R.O., Rodrigues, F.A. and Ramos, J.D., 2017. Effects of silicon on antioxidant enzymes, CO2, proline and biological activity of in vitro-grown cape gooseberry under salinity stress. Australian Journal of Crop Science, 11(4), p.438.
- 5
Ahmad, P., Ahanger, M.A., Alam, P., Alyemeni, M.N., Wijaya, L., Ali, S. and Ashraf, M., 2018. Silicon (Si) Supplementation Alleviates NaCl Toxicity in Mung Bean [Vigna radiata (L.) Wilczek] Through the Modifications of Physio-biochemical Attributes and Key Antioxidant Enzymes. Journal of Plant Growth Regulation, pp.1-13.
- 6
Ahmad, P., Jaleel, C.A. and Sharma, S., 2010. Antioxidant defense system, lipid peroxidation, proline-metabolizing enzymes, and biochemical activities in two Morus alba genotypes subjected to NaCl stress. Russian Journal of Plant Physiology, 57(4), pp.509-517.
- 7
Ahmad, S., Zhang, T.I.A.N.Z.H.E.N., Shaheen, T. and RAHMAN, M.U., 2007. Identifying genetic variation in Gossypium based on single nucleotide polymorphism. Pakistan Journal of Botany, 39(4), p.1245.
- 8
Alissa, E.M. and Ferns, G.A., 2012. Functional foods and nutraceuticals in the primary prevention of cardiovascular diseases. Journal of nutrition and metabolism, 2012.
- 9
Ahmad, P. and Umar, S., Role of Antioxidants in Plants, 2011. Studium Press, New Delhi, India.
- 10
Ashraf, M.F.M.R. and Foolad, M., 2007. Roles of glycine betaine and proline in improving plant abiotic stress resistance. Environmental and experimental botany, 59(2), pp.206-216.
- 11
Ashraf, M., Akram, N.A., Arteca, R.N. and Foolad, M.R., 2010. The physiological, biochemical and molecular roles of brassinosteroids and salicylic acid in plant processes and salt tolerance. Critical Reviews in Plant Sciences, 29(3), pp.162-190.
- 12
Ashraf, M.P.J.C. and Harris, P.J.C., 2004. Potential biochemical indicators of salinity tolerance in plants. Plant science, 166(1), pp.3-16.
- 13
Ashraf, M. and Harris, P. eds., 2005. Abiotic stresses: plant resistance through breeding and molecular approaches. CRC Press.
- 14
Ashraf, M.A., Ashraf, M. and Shahbaz, M., 2012. Growth stage-based modulation in antioxidant defense system and proline accumulation in two hexaploid wheat (Triticum aestivum L.) cultivars differing in salinity tolerance. Flora-Morphology, Distribution, Functional Ecology of Plants, 207(5), pp.388-397.
- 15
Ashraf, M.Y., Rafique, N., Ashraf, M., Azhar, N. and Marchand, M., 2013. Effect of supplemental potassium (K+) on growth, physiological and biochemical attributes of wheat grown under saline conditions. Journal of plant nutrition, 36(3), pp.443-458.
- 16
Ashraf, M.A., Akbar, A., Parveen, A., Rasheed, R., Hussain, I. and Iqbal, M., 2018. Phenological application of selenium differentially improves growth, oxidative defense and ion homeostasis in maize under salinity stress. Plant Physiology and Biochemistry, 123, pp.268-280.
- 17
Al-maskri, A., Hameed, M., Ashraf, M., Khan, M.M., Fatima, S., Nawaz, T. and Batool, R., 2014. Structural features of some wheat (Triticum spp.) landraces/ cultivars under drought and salt stress. Arid Land Research and Management, 28(3), pp.355-370.
- 18
Asgari, H.R., Cornelis, W. and Van Damme, P., 2012. Salt stress effect on wheat (Triticum aestivum L.) growth and leaf ion concentrations. International Journal of Plant Production, 6, pp. 195–208.
- 19
Anderson, J.V. and Davis, D.G., 2004. Abiotic stress alters transcript profiles and activity of glutathione S-transferase, glutathione peroxidase, and glutathione reductase in Euphorbia esula. Physiologia plantarum, 120(3), pp.421-433.
- 20
Bauder, J.W. and Brock, T.A., 1992. Crop species, amendment, and water quality effects on selected soil physical properties. Soil Science Society of America Journal, 56(4), pp.1292-1298.
- 21
Baskar, V., Venkatesh, R. and Ramalingam, S., 2018. Flavonoids (Antioxidants Systems) in Higher Plants and Their Response to Stresses. In Antioxidants and Antioxidant Enzymes in Higher Plants (pp. 253-268). Springer, Cham.
- 22
Broadbent P, Creissen GP, Kular B, Wellburn AR, Mullineaux PM (1995) Oxidative stress responses in transgenic tobacco containing altered levels of glutathione reductase activity. Plant Journal, 8, pp. 247–255.
- 23
Bor, M., Özdemir, F. and Türkan, I., 2003. The effect of salt stress on lipid peroxidation and antioxidants in leaves of sugar beet Beta vulgaris L. and wild beet Beta maritima L. Plant Science, 164(1), pp.77-84.
- 24
Bela, K., Horváth, E., Gallé, Á., Szabados, L., Tari, I. and Csiszár, J., 2015. Plant glutathione peroxidases: emerging role of the antioxidant enzymes in plant development and stress responses. Journal of Plant Physiology, 176, pp.192-201.
- 25
Cha-Um, S., Charoenpanich, A., Roytrakul, S. and Kirdmanee, C., 2009. Sugar accumulation, photosynthesis and growth of two indica rice varieties in response to salt stress. Acta physiologiae plantarum, 31(3), pp.477-486.
- 26
Chen, H. and Jiang, J.G., 2009. Osmotic responses of Dunaliella to the changes of salinity. Journal of cellular physiology, 219(2), pp.251-258.
- 27
Choudhury, F.K., Rivero, R.M., Blumwald, E. and Mittler, R., 2017. Reactive oxygen species, abiotic stress and stress combination. The Plant Journal, 90(5), pp.856-867.
- 28
Chen, H., Jiang, J.G. and Wu, G.H., 2009. Effects of salinity changes on the growth of Dunaliella salina and its isozyme activities of glycerol-3-phosphate dehydrogenase. Journal of agricultural and food chemistry, 57(14), pp.6178-6182.
- 29
Chen, Z., Cuin, T.A., Zhou, M., Twomey, A., Naidu, B.P. and Shabala, S., 2007. Compatible solute accumulation and stress-mitigating effects in barley genotypes contrasting in their salt tolerance. Journal of experimental botany, 58(15-16), pp.4245-4255.
- 30
Chołuj, D., Karwowska, R., Ciszewska, A. and Jasińska, M., 2008. Influence of long-term drought stress on osmolyte accumulation in sugar beet (Beta vulgaris L.) plants. Acta Physiologiae Plantarum, 30(5), p.679.
- 31
Chawla, S., Jain, S. and Jain, V., 2013. Salinity induced oxidative stress and antioxidant system in salt-tolerant and salt-sensitive cultivars of rice (Oryza sativa L.). Journal of plant biochemistry and biotechnology, 22(1), pp.27-34.
- 32
Chaves, M.M., Maroco, J.P. and Pereira, J.S., 2003. Understanding plant responses to drought—from genes to the whole plant. Functional plant biology, 30(3), pp.239-264.
- 33
Chakraborty, K., Bhaduri, D., Meena, H.N. and Kalariya, K., 2016. External potassium (K+) application improves salinity tolerance by promoting Na+-exclusion, K+-accumulation and osmotic adjustment in contrasting peanut cultivars. Plant Physiology and Biochemistry, 103, pp.143-153.
- 34
da COSTA, R.C.L., LOBATO, A.K.D.S., da SILVEIRA, J.A.G. and LAUGHINGHOUSE IV, H.D., 2011. ABA-mediated proline synthesis in cowpea leaves exposed to water deficiency and rehydration. Turkish Journal of Agriculture and Forestry, 35(3), pp.309-317.
- 35
Diao, Y., Xu, H., Li, G., Yu, A., Yu, X., Hu, W., Zheng, X., Li, S., Wang, Y. and Hu, Z., 2014. Cloning a glutathione peroxidase gene from Nelumbo nucifera and enhanced salt tolerance by overexpressing in rice. Molecular biology reports, 41(8), pp.4919-4927.
- 36
de Cássia Alves, R., de Medeiros, A.S., Nicolau, M.C.M., Neto, A.P., Lima, L.W., Tezotto, T. and Gratão, P.L., 2018. The partial root-zone saline irrigation system and antioxidant responses in tomato plants. Plant Physiology and Biochemistry, 127, pp.366-379.
- 37
Devi, S.R. and Prasad, M.N.V., 1998. Copper toxicity in Ceratophyllum demersum L.(Coontail), a free floating macrophyte: response of antioxidant enzymes and antioxidants. Plant science, 138(2), pp.157-165.
- 38
Dantas, B.F., Ribeiro, L.D.S. and Aragão, C.A., 2007. Germination, initial growth and cotyledon protein content of bean cultivars under salinity stress. Revista Brasileira de Sementes, 29(2), pp.106-110.
- 39
Das, K. and Roychoudhury, A., 2014. Reactive oxygen species (ROS) and response of antioxidants as ROS-scavengers during environmental stress in plants. Frontiers in Environmental Science, 2, p.53.
- 40
Dietz, K. J., Tavakoli N. and Kluge C., 1969.Significance of the V Type ATPase for the adaptation to stressful growth conditions and its regulation on the molecular and biochemical level. Journal of Experimental Botany, 363 (52), pp. 1969.
- 41
dos Reis, S.P., Lima, A.M. and de Souza, C.R.B., 2012. Recent molecular advances on downstream plant responses to abiotic stress. International Journal of Molecular Sciences, 13(7), pp.8628-8647.
- 42
Dugasa, M.T., Cao, F., Ibrahim, W. and Wu, F., 2018. Genotypic difference in physiological and biochemical characteristics in response to single and combined stresses of drought and salinity between the two wheat genotypes (Triticum aestivum) differing in salt tolerance. Physiologia plantarum.
- 43
Eggert, A., Nitschke, U., West, J.A., Michalik, D. and Karsten, U., 2007a. Acclimation of the intertidal red alga Bangiopsis subsimplex (Stylonematophyceae) to salinity changes. Journal of Experimental Marine Biology and Ecology, 343(2), pp.176-186.
- 44
Eggert, A., Raimund, S., Michalik, D., West, J. and Karsten, U., 2007b. Ecophysiological performance of the primitive red alga Dixoniella grisea (Rhodellophyceae) to irradiance, temperature and salinity stress: growth responses and the osmotic role of mannitol. Phycologia, 46(1), pp.22-28.
- 45
Ediga, A., Hemalatha, S. and Meriga, B., 2013. Effect of salinity stress on antioxidant defense system of two finger millet cultivars (Eleusine coracana (L.) Gaertn) differing in their sensitivity. Adv Biol Res, 7(5), pp.180-187.
- 46
FAO. 2015. Technical issues of salt-affected soils.
- 47
Foyer, C.H. and Noctor, G., 2011. Ascorbate and glutathione: the heart of the redox hub. Plant physiology, 155(1), pp.2-18.
- 48
Flowers, T.J. and Flowers, S.A., 2005. Why does salinity pose such a difficult problem for plant breeders?. Agricultural water management, 78(1-2), pp.15-24.
- 49
Flowers, T.J. and Yeo, A.R., 1995. Breeding for salinity resistance in crop plants: where next?. Functional Plant Biology, 22(6), pp.875-884.
- 50
Foolad, M.R., 2007. Genome mapping and molecular breeding of tomato. International journal of plant genomics, 2007.
- 51
García-Caparrós, P., Hasanuzzaman, M. and Lao, M.T., 2018. Ion Homeostasis and Antioxidant Defense Toward Salt Tolerance in Plants. In Plant Nutrients and Abiotic Stress Tolerance (pp. 415-436). Springer, Singapore.
- 52
Gharsallah, C., Fakhfakh, H., Grubb, D. and Gorsane, F., 2016. Effect of salt stress on ion concentration, proline content, antioxidant enzyme activities and gene expression in tomato cultivars. AoB Plants, 8.
- 53
Gao, S., Ouyang, C., Wang, S., Xu, Y., Tang, L. and Chen, F., 2008. Effects of salt stress on growth, antioxidant enzyme and phenylalanine ammonia-lyase activities in Jatropha curcas L. seedlings. Plant Soil Environ, 54(9), pp.374-381.
- 54
Gao, F., Chen, J., Ma, T., Li, H., Wang, N., Li, Z., Zhang, Z. and Zhou, Y., 2014. The glutathione peroxidase gene family in Thellungiella salsuginea: genome-wide identification, classification, and gene and protein expression analysis under stress conditions. International journal of molecular sciences, 15(2), pp.3319-3335.
- 55
Gagneul, D., Aïnouche, A., Duhazé, C., Lugan, R., Larher, F.R. and Bouchereau, A., 2007. A reassessment of the function of the so-called compatible solutes in the halophytic Plumbaginaceae Limonium latifolium. Plant Physiology, 144(3), pp.1598-1611.
- 56
Gelli, A., Higgins, V.J. and Blumwald, E., 1997. Activation of plant plasma membrane Ca2+-permeable channels by race-specific fungal elicitors. Plant Physiology, 113(1), pp.269-279.
- 57
Geebelen, W., Vangronsveld, J., Adriano, D.C., Van Poucke, L.C. and Clijsters, H., 2002. Effects of Pb‐EDTA and EDTA on oxidative stress reactions and mineral uptake in Phaseolus vulgaris. Physiologia plantarum, 115(3), pp.377-384.
- 58
Gill, S.S. and Tuteja, N., 2010. Reactive oxygen species and antioxidant machinery in abiotic stress tolerance in crop plants. Plant physiology and biochemistry, 48(12), pp.909-930.
- 59
Golkar, P. and Taghizadeh, M., 2018. In vitro evaluation of phenolic and osmolite compounds, ionic content, and antioxidant activity in safflower (Carthamus tinctorius L.) under salinity stress. Plant Cell, Tissue and Organ Culture (PCTOC), pp.1-12.
- 60
Gupta, D.K., Palma, J.M. and Corpas, F.J. eds., 2018. Antioxidants and Antioxidant Enzymes in Higher Plants. Springer.
- 61
GUL, H., ANJUM, L., ARIF, M., SHAH, M. and KHAN, A., 2018. effects of exogeneous application of putrescine on different biochemical parameters of Zea mays L. Under Salinity Stress. FUUAST Journal of Biology, 8(1).
- 62
Gupta, B. and Huang, B., 2014. Mechanism of salinity tolerance in plants: physiological, biochemical, and molecular characterization. International journal of genomics, 2014.
- 63
Greenway, H. and Munns, R., 1980. Mechanisms of salt tolerance in nonhalophytes. Annual review of plant physiology, 31(1), pp.149-190.
- 64
Gorham, J., 1992. Stress tolerance and mechanisms behind tolerance in barley. Barley Genetics VI, 2, pp.1035-1049.
- 65
Hare, P.D. and Cress, W.A., 1997. Metabolic implications of stress-induced proline accumulation in plants. Plant growth regulation, 21(2), pp.79-102.
- 66
Hasanuzzaman, M., Hossain, M.A., da Silva, J.A.T. and Fujita, M., 2012. Plant response and tolerance to abiotic oxidative stress: antioxidant defense is a key factor. In Crop stress and its management: Perspectives and strategies (pp. 261-315). Springer, Dordrecht.
- 67
Hasanuzzaman, M., Nahar, K. and Fujita, M., 2013. Plant response to salt stress and role of exogenous protectants to mitigate salt-induced damages. In Ecophysiology and responses of plants under salt stress (pp. 25-87). Springer, New York, NY.
- 68
Hassan, N.M., Serag, M.S. and El-Feky, F.M., 2004. Changes in nitrogen content and protein profiles following in vitro selection of NaCl resistant mung bean and tomato. Acta Physiologiae Plantarum, 26(2), p.165.
- 69
Hasegawa, P.M., Bressan, R.A., Zhu, J.K. and Bohnert, H.J., 2000. Plant cellular and molecular responses to high salinity. Annual review of plant biology, 51(1), pp.463-499.
- 70
Hasegawa, P.M., 2013. Sodium (Na+) homeostasis and salt tolerance of plants. Environmental and Experimental Botany, 92, pp.19-31.
- 71
Hauser, F. and Horie, T., 2010. A conserved primary salt tolerance mechanism mediated by HKT transporters: a mechanism for sodium exclusion and maintenance of high K+/Na+ ratio in leaves during salinity stress. Plant, cell & environment, 33(4), pp.552-565.
- 72
Hasanuzzaman, M., Nahar, K., Rohman, M.M., Anee, T.I., Huang, Y. and Fujita, M., 2018. Exogenous Silicon Protects Brassica napus Plants from Salinity-Induced Oxidative Stress Through the Modulation of AsA-GSH Pathway, Thiol-Dependent Antioxidant Enzymes and Glyoxalase Systems. Gesunde Pflanzen, pp.1-10.
- 73
Hellmann, H., Funck, D., Rentsch, D. and Frommer, W.B., 2000. Hypersensitivity of an Arabidopsis sugar signaling mutant toward exogenous proline application. Plant Physiology, 122(2), pp.357-368.
- 74
James, R.A., Blake, C., Byrt, C.S. and Munns, R., 2011. Major genes for Na+ exclusion, Nax1 and Nax2 (wheat HKT1; 4 and HKT1; 5), decrease Na+ accumulation in bread wheat leaves under saline and waterlogged conditions. Journal of experimental botany, 62(8), pp.2939-2947.
- 75
Jiang, C., Zu, C., Lu, D., Zheng, Q., Shen, J., Wang, H. and Li, D., 2017. Effect of exogenous selenium supply on photosynthesis, Na+ accumulation and antioxidative capacity of maize (Zea mays L.) under salinity stress. Scientific Reports, 7, p.42039.
- 76
Joseph, S., Derakhshani, Z., Murphy, D.J. and Bhave, M., 2017. Glycine betaine: biosynthesis, roles in abiotic stress tolerance of plants and significance as a nutraceutical. Agricultural research updates, Vol. 21 (series: Agricultural Research Updates)/Prathamesh Gorawala, Srushti Mandhatri (eds.), 5, p.183.
- 77
Karan, R. and Subudhi, P.K., 2012. A stress inducible SUMO conjugating enzyme gene (SaSce9) from a grass halophyte Spartina alterniflora enhances salinity and drought stress tolerance in Arabidopsis. BMC plant biology, 12(1), pp.187.
- 78
Karim B. H., Antonella C., Elkahoui S., Annamaria R. and Chedly A. 2007. Sea fennel (Crithmum maritimum L.) under salinity conditions: a comparison of leaf and root antioxidant responses. Plant Growth Regulation December 2007, 53(3), pp. 185.
- 79
Khan, M.A. and Rizvi, Y., 1994. Effect of salinity, temperature, and growth regulators on the germination and early seedling growth of Atriplex griffithii var. stocksii. Canadian Journal of Botany, 72(4), pp.475-479.
- 80
Khan, M.A. and Weber, D.J., 2006. Ecophysiology of high salinity tolerant plants (Vol. 40). Springer Science & Business Media.
- 81
Kishor, P.K., Sangam, S., Amrutha, R.N., Laxmi, P.S., Naidu, K.R., Rao, K.R.S.S., Rao, S., Reddy, K.J., Theriappan, P. and Sreenivasulu, N., 2005. Regulation of proline biosynthesis, degradation, uptake and transport in higher plants: its implications in plant growth and abiotic stress tolerance. Current science, pp.424-438.
- 82
Kim, Y.H., Khan, A.L., Waqas, M. and Lee, I.J., 2017. Silicon regulates antioxidant activities of crop plants under abiotic-induced oxidative stress: a review. Frontiers in plant science, 8, p.510.
- 83
Läuchli, A. and Epstein, E., 1990. Plant responses to saline and sodic conditions. Agricultural salinity assessment and management, 71, pp.113-137.
- 84
Larher, F., Rotival-Garnier, N., Lemesle, P., Plasman, M. and Bouchereau, A., 1996. The glycine betaine inhibitory effect on the osmoinduced proline response of rape leaf discs. Plant Science, 113(1), pp.21-31.
- 85
Lee, S., Choi, H., Suh, S., Doo, I.S., Oh, K.Y., Choi, E.J., Taylor, A.T.S., Low, P.S. and Lee, Y., 1999. Oligogalacturonic acid and chitosan reduce stomatal aperture by inducing the evolution of reactive oxygen species from guard cells of tomato and Commelina communis. Plant physiology, 121(1), pp.147-152.
- 86
Lira, R.M., Silva, Ê.F., Willadino, L., Oliveira Filho, R.A. and Andrade, G.R., 2018. Activity of antioxidative enzymes in watercress and Chinese cabbage plants grown under hydroponic system with brackish water. Horticultura Brasileira, 36(2), pp.205-210.
- 87
Liu, T. and Van Staden, J., 2001. Partitioning of carbohydrates in salt-sensitive and salt-tolerant soybean callus cultures under salinity stress and its subsequent relief. Plant Growth Regulation, 33(1), pp.13-17.
- 88
Liang, D., Shen, Y., Ni, Z., Wang, Q., Lei, Z., Xu, N., Deng, Q., Lin, L., Wang, J., Lv, X. and Xia, H., 2018. Exogenous Melatonin Application Delays Senescence of Kiwifruit Leaves by Regulating the Antioxidant Capacity and Biosynthesis of Flavonoids. Frontiers in plant science, 9, p.426.
- 89
López, M., Tejera, N.A., Iribarne, C., Lluch, C. and Herrera‐Cervera, J.A., 2008. Trehalose and trehalase in root nodules of Medicago truncatula and Phaseolus vulgaris in response to salt stress. Physiologia plantarum, 134(4), pp.575-582.
- 90
Luis, A., Corpas, F.J., López-Huertas, E. and Palma, J.M., 2018. Plant Superoxide Dismutases: Function Under Abiotic Stress Conditions. In Antioxidants and Antioxidant Enzymes in Higher Plants (pp. 1-26). Springer, Cham.
- 91
Ma, L., Zhang, H., Sun, L., Jiao, Y., Zhang, G., Miao, C. and Hao, F., 2011. NADPH oxidase AtrbohD and AtrbohF function in ROS-dependent regulation of Na+/K+ homeostasis in Arabidopsis under salt stress. Journal of Experimental Botany, 63(1), pp.305-317.
- 92
Martinez, V., Nieves-Cordones, M., Lopez-Delacalle, M., Rodenas, R., Mestre, T.C., Garcia-Sanchez, F., Rubio, F., Nortes, P.A., Mittler, R. and Rivero, R.M., 2018. Tolerance to stress combination in tomato plants: New insights in the protective role of melatonin. Molecules, 23(3), p.535.
- 93
Maghsoudi, K., Emam, Y., Niazi, A., Pessarakli, M. and Arvin, M.J., 2018. P5CS expression level and proline accumulation in the sensitive and tolerant wheat cultivars under control and drought stress conditions in the presence/absence of silicon and salicylic acid. Journal of Plant Interactions, 13(1), pp.461-471.
- 94
Merchant, A. and Adams, M., 2005. Stable osmotica in Eucalyptus spathulata—responses to salt and water deficit stress. Functional Plant Biology, 32(9), pp.797-805.
- 95
Munns, R. and Tester, M., 2008. Mechanisms of salinity tolerance. Annu. Rev. Plant Biol., 59, pp.651-681.Mian A, Oomen RJFJ, Isayenkov S, Sentenac H, Maathuis FJM, Very AA (2011a) Over-expression of an Na(+)- and K(+)-permeable HKT transporter in barley improves salt tolerance. Plant J 68: 468–479.
- 96
Mahdavi, B. and Rahimi, A., 2013. Seed priming with chitosan improves the germination and growth performance of ajowan (Carum copticum) under salt stress. EurAsian Journal of BioSciences, 7.
- 97
Munns, R., 2005. Genes and salt tolerance: bringing them together. New phytologist, 167(3), pp.645-663.
- 98
Munns, R., James, R.A., Xu, B., Athman, A., Conn, S.J., Jordans, C., Byrt, C.S., Hare, R.A., Tyerman, S.D., Tester, M. and Plett, D., 2012. Wheat grain yield on saline soils is improved by an ancestral Na+ transporter gene. Nature biotechnology, 30(4), p.360.
- 99
Munne-Bosch, S., 2005. The role of α-tocopherol in plant stress tolerance. Journal of plant physiology, 162(7), pp.743-748.
- 100
Munns, R. and Tester, M., 2008. Mechanisms of salinity tolerance. Annu. Rev. Plant Biol., 59, pp.651-681.
- 101
Mian, A.A., Senadheera, P. and Maathuis, F.J., 2011. Improving crop salt tolerance: anion and cation transporters as genetic engineering targets. Plant Stress, 5, pp.64-72.
- 102
Murshed, R., Lopez-Lauri, F. and Sallanon, H., 2014. Effect of salt stress on tomato fruit antioxidant systems depends on fruit development stage. Physiology and Molecular Biology of Plants, 20(1), pp.15-29.
- 103
Mguis, K., Albouchi, A., Abassi, M., Khadhri, A., Ykoubi-Tej, M., Mahjoub, A., Brahim, N.B. and Ouerghi, Z., 2013. Responses of leaf growth and gas exchanges to salt stress during reproductive stage in wild wheat relative Aegilops geniculata Roth. and wheat (Triticum durum Desf.). Acta physiologiae plantarum, 35(5), pp.1453-1461.
- 104
Morgan, J.M., 1984. Osmoregulation and water stress in higher plants. Annual review of plant physiology, 35(1), pp.299-319.
- 105
M. De Lourdes Oliveira Otoch, A. C. Menezes Sobreira, M. E. Farias De Arag˜ao, E. G. Orellano, M. Da Guia Silva Lima, and D. FernandesDeMelo, “Saltmodulation of vacuolarH+-ATPase and H+-Pyrophosphatase activities in Vigna unguiculata,” Journal of Plant Physiology, vol. 158, no. 5, pp. 545–551, 2001.
- 106
Mahajan, S. and Tuteja, N., 2005. Cold, salinity and drought stresses: an overview. Archives of biochemistry and biophysics, 444(2), pp.139-158.
- 107
Mittova, V., Guy, M., Tal, M. and Volokita, M., 2004. Salinity up-regulates the antioxidative system in root mitochondria and peroxisomes of the wild salt-tolerant tomato species Lycopersicon pennellii. Journal of experimental botany, 55(399), pp.1105-1113.
- 108
Mittova, V., Tal, M., Volokita, M. and Guy, M., 2003. Up-regulation of the leaf mitochondrial and peroxisomal antioxidative systems in response to salt-induced oxidative stress in the wild salt-tolerant tomato species Lycopersicon pennellii. Plant, Cell & Environment, 26(6), pp.845-856.
- 109
Mittova, V., Volokita, M. and Guy, M., 2015. Antioxidative systems and stress tolerance: insight from wild and cultivated tomato species. In Reactive oxygen and nitrogen species signaling and communication in plants (pp. 89-131). Springer, Cham.
- 110
Nahar, K., Hasanuzzaman, M., Alam, M.M. and Fujita, M., 2015. Roles of exogenous glutathione in antioxidant defense system and methylglyoxal detoxification during salt stress in mung bean. Biologia plantarum, 59(4), pp.745-756.
- 111
Niu, X., Bressan, R.A., Hasegawa, P.M. and Pardo, J.M., 1995. Ion homeostasis in NaCl stress environments. Plant physiology, 109(3), p.735.
- 112
Nikalje, G.C., Variyar, P.S., Joshi, M.V., Nikam, T.D. and Suprasanna, P., 2018. Temporal and spatial changes in ion homeostasis, antioxidant defense and accumulation of flavonoids and glycolipid in a halophyte Sesuvium portulacastrum (L.) L. PloS one, 13(4), p.e0193394.
- 113
Oh, D.H., Lee, S.Y., Bressan, R.A., Yun, D.J. and Bohnert, H.J., 2010. Intracellular consequences of SOS1 deficiency during salt stress. Journal of Experimental Botany, 61(4), pp.1205-1213.
- 114
Othman, Y., Al-Karaki, G., Al-Tawaha, A.R. and Al-Horani, A., 2006. Variation in germination and ion uptake in barley genotypes under salinity conditions. World Journal of Agricultural Sciences, 2(1), pp.11-15.
- 115
Otoch, M.D.L.O., Sobreira, A.C.M., de Aragão, M.E.F., Orellano, E.G., Lima, M.D.G.S. and de Melo, D.F., 2001. Salt modulation of vacuolar H+-ATPase and H+-Pyrophosphatase activities in Vigna unguiculata. Journal of Plant Physiology, 158(5), pp.545-551.
- 116
Patakas, A., Nikolaou, N., Zioziou, E., Radoglou, K. and Noitsakis, B., 2002. The role of organic solute and ion accumulation in osmotic adjustment in drought-stressed grapevines. Plant science, 163(2), pp.361-367.
- 117
Pessarakli, M., 2014. Handbook of plant and crop physiology. CRC Press.
- 118
Pottosin, I., Velarde-Buendía, A.M., Bose, J., Zepeda-Jazo, I., Shabala, S. and Dobrovinskaya, O., 2014. Cross-talk between reactive oxygen species and polyamines in regulation of ion transport across the plasma membrane: implications for plant adaptive responses. Journal of Experimental Botany, 65(5), pp.1271-1283.
- 119
Poustini, K., Siosemardeh, A. and Ranjbar, M., 2007. Proline accumulation as a response to salt stress in 30 wheat (Triticum aestivum L.) cultivars differing in salt tolerance. Genetic Resources and Crop Evolution, 54(5), pp.925-934.
- 120
Qadir, M., Quillérou, E., Nangia, V., Murtaza, G., Singh, M., Thomas, R.J., Drechsel, P. and Noble, A.D., 2014, November. Economics of salt-induced land degradation and restoration. In Natural Resources Forum (Vol. 38, No. 4, pp. 282-295).
- 121
Qureshi, M.I., Abdin, M.Z., Ahmad, J. and Iqbal, M., 2013. Effect of long-term salinity on cellular antioxidants, compatible solute and fatty acid profile of Sweet Annie (Artemisia annua L.). Phytochemistry, 95, pp.215-223.
- 122
Qureshi, T.M., Bano, A. and Ashraf, M.Y., 2015. Glycine Betaine and Proline Production in Eucalyptus Plant under NaCl Harassing Environment. Nucleus (Islamabad), 52(2), pp.88-97.
- 123
Raza, S.H., Athar, H.R., Ashraf, M. and Hameed, A., 2007. Glycinebetaine-induced modulation of antioxidant enzymes activities and ion accumulation in two wheat cultivars differing in salt tolerance. Environmental and Experimental Botany, 60(3), pp.368-376.
- 124
Rakhmankulova, Z.F., Shuyskaya, E.V., Shcherbakov, A.V., Fedyaev, V.V., Biktimerova, G.Y., Khafisova, R.R. and Usmanov, I.Y., 2015. Content of proline and flavonoids in the shoots of halophytes inhabiting the South Urals. Russian journal of plant physiology, 62(1), pp.71-79.
- 125
Rajendran, K., Tester, M. and Roy, S.J., 2009. Quantifying the three main components of salinity tolerance in cereals. Plant, cell & environment, 32(3), pp.237-249.
- 126
Rasheed, R., 2009. Salinity and extreme temperature effects on sprouting buds of sugarcane (Saccharum officinarum L.): some histological and biochemical studies (Doctoral dissertation, UNIVERSITY OF AGRICULTURE, FAISALABAD PAKISTAN).
- 127
Rahnama, A., James, R.A., Poustini, K. and Munns, R., 2010. Stomatal conductance as a screen for osmotic stress tolerance in durum wheat growing in saline soil. Functional Plant Biology, 37(3), pp.255-263.
- 128
Rozema, J. and Flowers, T., 2008. Crops for a salinized world. Science, pp.1478-1480.
- 129
Ruiz-Lozano, J.M., Porcel, R., Calvo-Polanco, M. and Aroca, R., 2018. Improvement of Salt Tolerance in Rice Plants by Arbuscular Mycorrhizal Symbiosis. In Root Biology (pp. 259-279). Springer, Cham.
- 130
Serrano, R., Mulet, J.M., Rios, G., Marquez, J.A., De Larrinoa, I.F., Leube, M.P., Mendizabal, I., Pascual-Ahuir, A., Proft, M., Ros, R. and Montesinos, C., 1999. A glimpse of the mechanisms of ion homeostasis during salt stress. Journal of experimental botany, pp.1023-1036.
- 131
Sanders, D., 2000. Plant biology: the salty tale of Arabidopsis. Current Biology, 10(13), pp.R486-R488.
- 132
Saha, P., Chatterjee, P. and Biswas, A.K., 2010. NaCl pretreatment alleviates salt stress by enhancement of antioxidant defense system and osmolyte accumulation in mungbean (Vigna radiata L. Wilczek).
- 133
Saad, A.S.I., Li, X., Li, H.P., Huang, T., Gao, C.S., Guo, M.W., Cheng, W., Zhao, G.Y. and Liao, Y.C., 2013. A rice stress-responsive NAC gene enhances tolerance of transgenic wheat to drought and salt stresses. Plant Science, 203, pp.33-40.
- 134
Sairam, R.K. and Tyagi, A., 2004. Physiological and molecular biology of salinity stress tolerance in deficient and cultivated genotypes of chickpea. Plant Growth Regul, 57(10).
- 135
Shabala, S. and Cuin, T.A., 2008. Potassium transport and plant salt tolerance. Physiologia Plantarum, 133(4), pp.651-669.
- 136
Souid, A., Bellani, L., Magné, C., Zorrig, W., Smaoui, A., Abdelly, C., Longo, V. and Hamed, K.B., 2018. Physiological and antioxidant responses of the sabkha biotope halophyte Limonium delicatulum to seasonal changes in environmental conditions. Plant Physiology and Biochemistry, 123, pp.180-191.
- 137
Sofo, A., Scopa, A., Nuzzaci, M. and Vitti, A., 2015. Ascorbate peroxidase and catalase activities and their genetic regulation in plants subjected to drought and salinity stresses. International journal of molecular sciences, 16(6), pp.13561-13578.
- 138
Shabala, S., Shabala, S., Cuin, T.A., Pang, J., Percey, W., Chen, Z., Conn, S., Eing, C. and Wegner, L.H., 2010. Xylem ionic relations and salinity tolerance in barley. The Plant Journal, 61(5), pp.839-853.
- 139
Ray, S.R., Bhuiyan, M.J.H., Anowar, M., Hossain, S.M. and Tahjib-Ul-Arif, M., 2015. Chitosan Suppresses Antioxidant Enzyme Activities for Mitigating Salt Stress in Mungbean Varieties. IOSR Journal of Agriculture and Veterinary Science, 9 (9), PP. 36-41.
- 140
Shigeoka, S., Ishikawa, T., Tamoi, M., Miyagawa, Y., Takeda, T., Yabuta, Y. and Yoshimura, K., 2002. Regulation and function of ascorbate peroxidase isoenzymes. Journal of experimental botany, 53(372), pp.1305-1319.
- 141
Shi, H., Ishitani, M., Kim, C. and Zhu, J.K., 2000. The Arabidopsis thaliana salt tolerance gene SOS1 encodes a putative Na+/H+ antiporter. Proceedings of the national academy of sciences, 97(12), pp.6896-6901.
- 142
Shi, H., Quintero, F.J., Pardo, J.M. and Zhu, J.K., 2002. The putative plasma membrane Na+/H+ antiporter SOS1 controls long-distance Na+ transport in plants. The Plant Cell, 14(2), pp.465-477.
- 143
Sudhakar, C., Lakshmi, A. and Giridarakumar, S., 2001. Changes in the antioxidant enzyme efficacy in two high yielding genotypes of mulberry (Morus alba L.) under NaCl salinity. Plant Science, 161(3), pp.613-619.
- 144
Su, J., Hirji, R., Zhang, L., He, C., Selvaraj, G. and Wu, R., 2006. Evaluation of the stress-inducible production of choline oxidase in transgenic rice as a strategy for producing the stress-protectant glycine betaine. Journal of Experimental Botany, 57(5), pp.1129-1135.
- 145
Tarczynski, M.C., Jensen, R.G. and Bohnert, H.J., 1993. Stress protection of transgenic tobacco by production of the osmolyte mannitol. Science, 259(5094), pp.508-510.
- 146
Talbi, S., Romero-Puertas, M.C., Hernández, A., Terrón, L., Ferchichi, A. and Sandalio, L.M., 2015. Drought tolerance in a Saharian plant Oudneya africana: role of antioxidant defences. Environmental and Experimental Botany, 111, pp.114-126.
- 147
Taïbi, K., Taïbi, F., Abderrahim, L.A., Ennajah, A., Belkhodja, M. and Mulet, J.M., 2016. Effect of salt stress on growth, chlorophyll content, lipid peroxidation and antioxidant defence systems in Phaseolus vulgaris L. South African Journal of Botany, 105, pp.306-312.
- 148
Tavakkoli, E., Rengasamy, P. and McDonald, G.K., 2010. High concentrations of Na+ and Cl–ions in soil solution have simultaneous detrimental effects on growth of faba bean under salinity stress. Journal of experimental botany, 61(15), pp.4449-4459.
- 149
Volkmar, K.M., Hu, Y. and Steppuhn, H., 1998. Physiological responses of plants to salinity: a review. Canadian journal of plant science, 78(1), pp.19-27.
- 150
Van Breusegem, F., Vranová, E., Dat, J.F. and Inzé, D., 2001. The role of active oxygen species in plant signal transduction. Plant Science, 161(3), pp.405-414.
- 151
Vílchez, J.I., Niehaus, K., Dowling, D.N., González-López, J. and Manzanera, M., 2018. Protection of Pepper Plants from Drought by Microbacterium sp. 3J1 by Modulation of the Plant’s Glutamine and α-ketoglutarate Content: A Comparative Metabolomics Approach. Frontiers in Microbiology, 9, p.284.
- 152
Volaire, F., Thomas, H. and Lelievre, F., 1998. Survival and recovery of perennial forage grasses under prolonged Mediterranean drought: I. Growth, death, water relations and solute content in herbage and stubble. The New Phytologist, 140(3), pp.439-449.
- 153
Wang, B., Lüttge, U. and Ratajczak, R., 2001. Effects of salt treatment and osmotic stress on V-ATPase and V-PPase in leaves of the halophyte Suaeda salsa. Journal of Experimental Botany, 52(365), pp.2355-2365.
- 154
Wang, W.B., Kim, Y.H., Lee, H.S., Kim, K.Y., Deng, X.P. and Kwak, S.S., 2009. Analysis of antioxidant enzyme activity during germination of alfalfa under salt and drought stresses. Plant Physiology and Biochemistry, 47(7), pp.570-577.
- 155
Willekens, H., Chamnongpol, S., Davey, M., Schraudner, M., Langebartels, C., Van Montagu, M., Inzé, D. and Van Camp, W., 1997. Catalase is a sink for H2O2 and is indispensable for stress defence in C3 plants. The EMBO journal, 16(16), pp.4806-4816.
- 156
Wahid, A.B.D.U.L., Rasul, E.J.A.Z. and Rao, A.U.R., 1999. Germination of seeds and propagules under salt stress. Handbook of plant and crop stress, 2, pp.153-167.
- 157
Yeo, A.R., 1983. Salinity resistance: physiologies and prices. Physiologia plantarum, 58(2), pp.214-222.
- 158
Zeng, F., Shabala, S., Dragišić Maksimović, J., Maksimović, V., Bonales-Alatorre, E., Shabala, L., Yu, M., Zhang, G. and Živanović, B.D., 2018. Revealing mechanisms of salinity tissue tolerance in succulent halophytes: a case study for Carpobrotus rossi. Plant, cell & environment.
- 159
Zhu, J.K., 2001. Cell signaling under salt, water and cold stresses. Current opinion in plant biology, 4(5), pp.401-406.
- 160
Zhu, X.Y., Jing, Y., Chen, G.C., Wang, S.M. and Zhang, C.L., 2003. Solute levels and osmoregulatory enzyme activities in reed plants adapted to drought and saline habitats. Plant growth regulation, 41(2), pp.165-172.
- 161
Zhang, J., Nishimura, N., Okubo, A. and Yamazaki, S., 2002. Development of an analytical method for the determination of betaines in higher plants by capillary electrophoresis at low pH. Phytochemical Analysis: An International Journal of Plant Chemical and Biochemical Techniques, 13(4), pp.189-194.
- 162
Zhang, Y., Zhong, J. and Xu, L., 2013. Identification and biochemical characterization of 20S proteasome in wheat roots under salt stress. Journal of plant biochemistry and biotechnology, 22(1), pp.62-70.
- 163
Zhao, X., Wei, P., Liu, Z., Yu, B. and Shi, H., 2017. Soybean Na+/H+ antiporter GmsSOS1 enhances antioxidant enzyme activity and reduces Na+ accumulation in Arabidopsis and yeast cells under salt stress. Acta Physiologiae Plantarum, 39(1), p.19.
Cited by 4#
- A Fusarium Isolate from a Salt Marsh Improves the Salinity Tolerance of a Commercial Cultivar of Festuca rubra via Enhanced Root K+ HomeostasisL. Wang, S. Munikumar, J. Yi et al.Microorganisms · 2026 · doi.org/10.3390/microorganisms14071598
- Effects of Combined Drought and Salinity Stress on Oxidative Damage and the Antioxidant Enzyme System in Aronia (Aronia melanocarpa L.) ‘Nero’ under In Vitro ConditionsÇ. KayaANADOLU JOURNAL OF AGRICULTURAL SCIENCES · 2026 · doi.org/10.7161/omuanajas.1900528
- Nano-chitosan-mediated salinity tolerance in Calendula officinalis: Nonlinear physiological thresholds and antioxidant responses identified via interpretable hybrid modelingA. Taheri-Garavand, Z. Bolhassani, A. Ahmadi et al.Current Plant Biology · 2026 · doi.org/10.1016/j.cpb.2026.100685
- Impact of Salinity Stress on Major Cereal Crops and Integrated Management Strategies for Sustainable ProductionU. Ali, S. Shah, M. Khaskheli et al.Journal of Applied Research in Plant Sciences · 2025 · doi.org/10.38211/joarps.2025.06.328
Each citation is confirmed in the citing article's own reference list (Crossref).